How an RNA m6A mark may help keep transposable elements active
Published:
Some of the most interesting biology happens at the borders between familiar categories. We often think of RNA as a message copied from DNA, and DNA methylation as a mark that helps control which genes are active. A recent presentation on LTR7 transposable elements in human pluripotent stem cells connects those ideas: an RNA modification may help recruit a DNA-modifying enzyme back to the genomic region that produced the RNA.
The idea is striking because it makes the transcript more than a by-product of an active DNA element. In the model presented, a chemical mark on LTR7 RNA is recognized by a protein that helps maintain an active chromatin environment at LTR7 itself. Here is how the researchers built that model, and what makes it compelling.
First, what is LTR7?
LTR7 is a family of long terminal repeat (LTR) sequences derived from endogenous retroelements. These sequences are part of the human genome, and some can function as regulatory DNA. In human pluripotent stem cells, LTR7 elements are active and associated with transcriptional regulators and co-activators. Their activity generally decreases as cells differentiate.
That makes LTR7 an intriguing place to study cell identity. But repeated elements occur in many copies across the genome, which creates a practical challenge: how do you identify proteins associated with a particular family of genomic regions?
Finding proteins at repetitive DNA
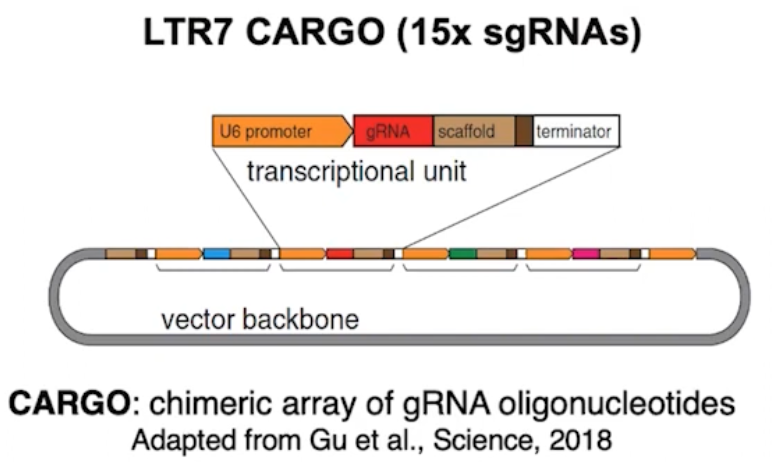
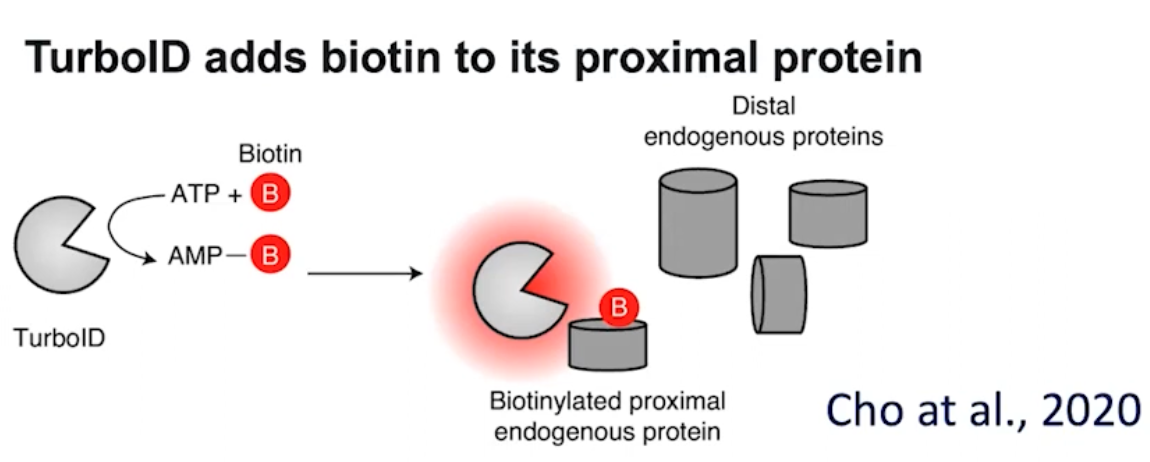
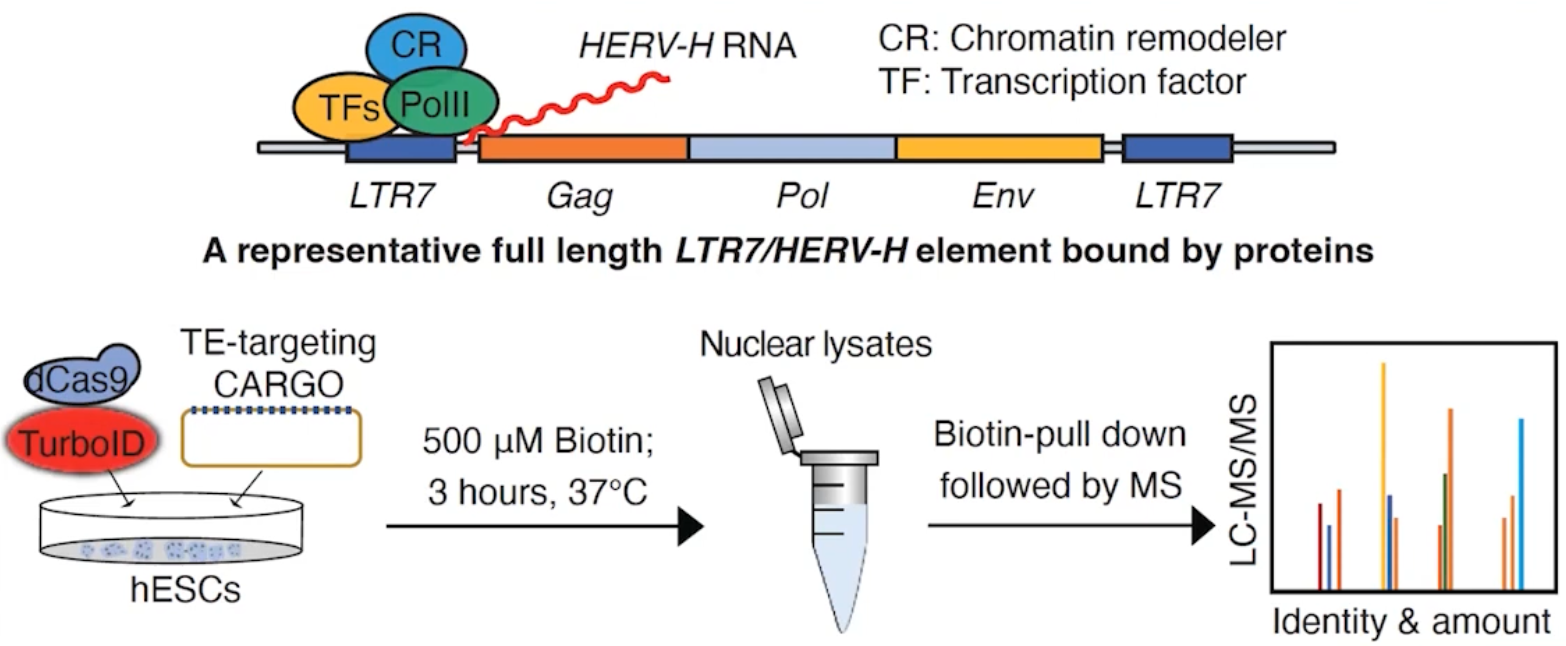
The team used CARGO-TurboID, a targeted proximity-labeling approach. Guide RNAs direct catalytically inactive Cas9 (dCas9) to many copies of LTR7. TurboID, attached to dCas9, adds a biotin tag to nearby proteins. Those tagged proteins can then be enriched and identified by mass spectrometry.
This is not a readout of every molecule touching LTR7 at every moment; it is a way to generate a neighborhood-level map. The researchers reported more than 140 proteins enriched at LTR7-associated regions, including YTHDC2, a protein known to recognize N6-methyladenosine (m6A) on RNA.
The proposed RNA-to-DNA connection
The researchers found that YTHDC2 is associated with m6A-modified LTR7 transcripts. m6A is a chemical modification added to RNA; proteins called m6A readers recognize it and can influence the RNA’s fate or interactions. The presentation links YTHDC2 to TET1, an enzyme that oxidizes 5-methylcytosine (5mC) in DNA, initiating pathways that can lead to DNA demethylation.
In the model, YTHDC2 helps bring TET1 to LTR7-associated regions. TET1 converts 5mC first to 5-hydroxymethylcytosine (5hmC) and can continue oxidizing it; 5hmC is therefore an intermediate and a measurable DNA modification, not simply another name for unmethylated DNA. The proposed outcome is a local environment less favorable to stable silencing.
The connection is suggestive, but it is worth describing precisely: the results support a pathway linking m6A-marked RNA, YTHDC2, TET1, and LTR7 chromatin. They do not mean that m6A itself is a DNA mark, or that every RNA transcript acts as a general-purpose guide to its matching genomic sequence.
What changes when YTHDC2 is depleted?
The perturbation experiments provide the clearest test of the model. When YTHDC2 was depleted, LTR7 transcription decreased. The chromatin changes were consistent with repression: the active-associated histone mark H3K27ac declined, while the repressive mark H3K9me3 increased. The researchers also reported increased 5mC and decreased 5hmC at the relevant regions, alongside reduced TET1 association.
Taken together, these observations connect an RNA-binding protein to both DNA modification and histone state. They also suggest that active LTR7 elements are not maintained by transcription alone; their transcripts may participate in a feedback relationship with the chromatin environment.
The presentation also links LTR7 activity and YTHDC2 to neuronal differentiation. That is an important biological consequence to investigate, but it should not be read as proof that LTR7 alone determines cell fate. Differentiation is controlled by many interacting pathways, and the reported results point to a contribution within that larger network.
Why this study caught my attention
The memorable part is the direction of the proposed conversation. DNA produces RNA, but the modified RNA may then help recruit a protein that influences the DNA’s local epigenetic state. It is a useful reminder that gene regulation is not always a one-way flow from genome to transcript.
The method matters, too. CARGO-TurboID offers a way to ask which proteins gather around repetitive genomic elements that are difficult to study one copy at a time. It does not settle every mechanistic question, but it creates a route from an interesting locus to testable candidate proteins.
The next questions are the ones I would want to see answered: which LTR7 RNA molecules are required for TET1 recruitment, how directly YTHDC2 interacts with TET1, and whether this pathway operates similarly across different pluripotent cell lines or during normal development. Answering them would sharpen the model from a compelling association-and-perturbation story into a more complete account of cause and effect.
For now, the takeaway is a carefully bounded one: in the presented experiments, m6A recognition by YTHDC2 is linked to TET1-associated DNA modification and active chromatin at LTR7 elements in human pluripotent stem cells. It is a vivid example of how RNA chemistry may help shape the chromatin context from which that RNA came.